




🚀 $RKLB | Wall Street Price Targets
🎯 Average: $102.15 | High: $150
📊 18 Buy | 4 Hold | 0 Sell
Top Analyst Targets:
• Stifel: $132
• Cantor Fitzgerald: $122
• Needham: $120
• Roth MKM: $110
• Morgan Stanley: $105
• Citi: $105
Neutron is the next big catalyst. 🚀
Let's Go! #RocketLab

🚨 $ONDS Q3 earnings are on deck.
📅 November 12, 2026
⏰ 8:30 AM ET
All eyes on revenue growth, backlog, new contracts, and 2027 guidance.
BULLISH! #ONDAS 🚀
Press Release: ir.ondas.com/press-releases/…


Ondas will report Q3 2026 financial results on November 12, 2026. Management will host a conference call and live webcast at 8:30 a.m. ET, followed by Q&A. $ONDS
ondas.com/post/ondas-to-repo…

One of the better frameworks I’ve seen for why proteoform level proteomics could actually change oncology.
Network redundancy, multi-node targeting, and the $NAUT angle. Worth reading.

For the purpose of understanding $NAUT's potential to revolutionise Oncology, consider the following mental framework: cancer is in fact a dysregulated molecular signalling network, on a first principles basis.
The human body operates through molecular signalling networks that tell cells when to grow, divide, survive, repair themselves or die.
Cancer emerges when mutations and other regulatory abnormalities disrupt these networks, allowing cells to override the instructions that normally keep them under control.
Consider six important nodes in this network:
1/ EGFR: the upstream growth receptor.
EGFR sits on the cell membrane and receives growth signals from outside the cell. When activated, it changes its molecular configuration, becomes phosphorylated at specific amino acid positions and initiates downstream signalling.
Two major pathways branch from EGFR: KRAS–MAPK and PI3K–AKT.
The former primarily regulates proliferation, while the latter coordinates growth, metabolism and survival. Both can become pathologically active in cancer.
2/ KRAS: the molecular growth switch.
KRAS is essentially a binary switch, cycling between inactive GDP-bound and active GTP-bound states.
When activated, it triggers a cascade:
KRAS → RAF → MEK → ERK → proliferation.
ERK ultimately regulates proteins and transcription factors that tell the cell to divide.
Mutations such as KRAS G12D can disrupt the switch's normal regulation, allowing proliferative signals to persist even without continuous upstream stimulation.
This is particularly relevant to pancreatic cancer, where KRAS mutations occur in approximately 90–95% of pancreatic ductal adenocarcinomas.
3/ PI3K: the parallel survival pathway.
EGFR can also activate PI3K, which converts the membrane lipid PIP2 into PIP3.
PIP3 recruits proteins such as AKT1 to the membrane, facilitating their activation.
The important point is that a cancer cell can maintain survival signalling through PI3K–AKT even when the KRAS–MAPK branch is inhibited.
This creates redundancy in the network.
And redundancy makes cancer considerably harder to kill.
4/ PTEN: the molecular brake.
PTEN reverses the reaction catalysed by PI3K, converting PIP3 back into PIP2.
It therefore restrains downstream AKT activation.
When PTEN is lost or inactivated, this brake disappears. The PI3K–AKT pathway can remain abnormally active, allowing malignant cells to survive signals that would otherwise trigger programmed cell death.
Importantly, cancer is not exclusively the result of activating growth-promoting genes. It can also result from disabling the molecular machinery that normally suppresses them.
5/ AKT1: the survival and growth controller.
AKT1 sits downstream of PI3K and regulates several fundamental cellular functions through proteins including mTOR, FOXO and GSK3.
But AKT1 is not simply ON or OFF because the protein exists.
Its activity depends on its molecular state.
Two particularly important phosphorylation sites are T308 and S473. Their phosphorylation helps determine AKT1 activation and downstream signalling.
This is where the proteoform thesis becomes interesting.
Measuring the abundance of AKT1 is not equivalent to determining the precise combination of modifications present on AKT1 molecules.
And those combinations can materially affect what the protein does.
6/ STAT3: an additional survival programme.
STAT3 is a transcription factor that can be activated by inflammatory cytokines, JAK kinases and growth-factor signalling.
When activated, STAT3 regulates genes involved in survival, proliferation, inflammation and immune evasion.
This provides cancer cells with another mechanism for maintaining malignant behaviour, potentially even when other signalling pathways are pharmacologically suppressed.
Now consider the problem from a systems perspective.
We have an interconnected network of molecular switches, feedback loops, inhibitory mechanisms and alternative survival pathways.
Some mutations increase the activity of particular nodes. Others disable the brakes. And still others alter how the network responds to therapeutic intervention.
The central problem in Oncology is therefore not merely identifying which genes are mutated. It is understanding the molecular configuration that allows the entire malignant network to remain operational.
This brings us to Mariano Barbacid.
His team's experimental pancreatic cancer work illustrates precisely why this framework matters.
Rather than inhibiting KRAS in isolation, the researchers combined interventions against KRAS, EGFR and STAT3, simultaneously disrupting multiple mechanisms supporting the malignant state.
The combination produced durable tumour regression in preclinical mouse models.
It is not yet proof that the same strategy will cure human pancreatic cancer. But the conceptual implication is enormous.
Sometimes disabling a single oncogenic protein is insufficient because the network can compensate.
Disrupting several critical dependencies simultaneously can produce a fundamentally different outcome.
Now imagine being able to read the molecular state of that network rather than infer it primarily from DNA mutations.
This is where I believe $NAUT could become extraordinarily important.
DNA sequencing tells us what the genomic instructions look like.
RNA sequencing tells us which instructions are being transcribed.
Traditional proteomics tells us something about the proteins that are present and, depending on the method, certain molecular modifications.
But the actual biological machinery operates through proteins whose functions depend on their precise molecular configurations.
Phosphorylation, cleavage, acetylation, ubiquitination and other post-translational modifications can change a protein's activity, localization, interactions, stability or degradation.
And multiple modifications can coexist on the same protein molecule.
These distinct molecular configurations are called proteoforms.
The important distinction is between knowing that a protein is present, knowing that particular modifications exist somewhere in a sample, and knowing which modifications coexist on the same intact protein.
Those are not equivalent measurements.
For example, detecting AKT1 phosphorylation at T308 and S473 separately does not automatically tell us how frequently both modifications coexist on the same AKT1 molecule.
A platform capable of resolving these combinations could provide a much richer picture of the molecular states governing cellular behaviour.
That is the central technological promise I see in Nautilus.
And it leads to the next step in the thesis.
Suppose we measure a tumour's initial proteoform configuration.
We then administer a drug or combination of drugs.
After treatment, we measure the new molecular state.
We now have a data pair:
Initial molecular state + intervention → final molecular state.
Repeat this across thousands of proteins, many interventions and eventually large numbers of patients, with clinical outcomes attached.
The resulting dataset could teach AI how biological signalling networks respond to therapeutic interventions.
Instead of simply associating a mutation with an approved drug, we could begin modelling the molecular state transitions that determine whether a tumour proliferates, regresses or develops resistance.
The objective would be to identify the smallest effective combination of interventions that moves the network away from the malignant state and towards sustained tumour suppression, while preserving healthy tissue.
In the Barbacid example, the relevant intervention nodes were KRAS, EGFR and STAT3.
In another tumour, the critical combination might involve PI3K, AKT, MEK, an immune signalling pathway or entirely different molecular mechanisms.
The optimal combination is a property of the tumour's specific molecular state, not necessarily a universal recipe for a particular cancer.
This is why the opportunity extends far beyond a single cancer type.
The EGFR–KRAS–PI3K–AKT–STAT3 network is merely a small subset of the machinery involved in cancer. The complete ontology also includes DNA repair, epigenetic regulation, metabolism, apoptosis, immune evasion, cellular senescence and interactions with the tumour microenvironment.
A sufficiently comprehensive molecular-state model could eventually connect these systems.
Of course, Nautilus has not demonstrated the ability to map every clinically relevant cancer proteoform, infer every signalling dependency or prescribe curative drug combinations. Those are enormous scientific, computational and clinical challenges.
But consider the direction of travel.
Genomics gave us a map of the instructions.
Proteoform-resolved proteomics could give us a much more detailed picture of the machinery executing those instructions.
And AI could eventually learn how to manipulate that machinery by observing what happens before and after intervention.
My $NAUT thesis is that the company is building a potentially critical measurement layer for this transition: from reading biological instructions to reading biological states, and eventually learning how to change them.
If this works, the opportunity is not simply better cancer diagnostics.
It is the possibility of turning Oncology from a largely mutation-guided treatment discipline into a more comprehensive, predictive science of molecular network control.
And cancer is only one application of that idea.

$ONDS on the Move. ⚡️
Logistics UGV that doesn’t care about the terrain. Ark Robotics (Estonia) bringing the M4 to UGV MUDDER — Dec 2, Tallinn

#UGVMUDDER2026 Meet the Teams: Ark Robotics from #Estonia brings its M4 logistics UGV to UGV MUDDER. Up to 200 kg payload, mission-ready in 10 minutes.
December 2 · Tallinn
Register your UGV or attend as a visitor: ugv-mudder.ondascapital.com/…
#OndasCapital #UGV #DefenceTech
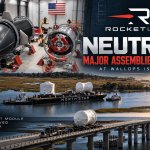
🚀 $RKLB NEUTRON UPDATE
Another milestone for Rocket Lab!
Neutron's Stage 2 and Thrust Module have arrived at Wallops Island, Virginia.
Next up: integrated fluids testing, launch mount interface checks, and Stage 2 testing.
One step closer to the launch pad. 🚀🔥


Neutron’s Stage 2 and Thrust Module have arrived to Virginia. After a short barge ride from the Neutron Factory, these major assemblies have now been offloaded on Wallops Island and are going through arrival checkouts.
Next up: integrated fluids testing and launch mount interface checkouts for the Thrust Module, with Stage 2 to follow on the test stand beside it soon after.


Picked up 12,000 shares of $NAUT on Monday at $2.46.
Small, high-risk speculative bet on the future of proteomics. Jeff Bezos' investment firm, Bezos Expeditions, was an early backer. That caught my curiosity. @cyberprince_rwo relentless posting kept it on my radar.
Could go to zero. Don't care. I'm comfortable with the risk.
Do your own research. Don't follow me into trades.


$ONDS on the Move! ⚡️
A robot went down in Ukraine. Another robot went back to rescue it. Both made it home.
Robots rescuing robots. Science fiction is becoming reality. 🤖
The future of autonomous defense is already here.

A ground robot in Ukraine’s Sumy region stopped working mid-mission. Its unit sent a second robot to bring it back, and both made it home.
Robots helping robots is no longer science fiction.
What should builders hear more often from the people who use their systems?
#UGV #UnmannedSystems

$RKLB SDA Tranche 2 satellite production in full swing at Rocket Lab — 8 of 18 spacecraft on the floor right now. 🛰️
Let's Dance! $RKLB 🚀
Members of @SemperCitiusSDA's Tranche 2 leadership team were recently at Rocket Lab's California headquarters to see T2TL-Beta in production.
Eight of 18 spacecraft are on the floor right now, in build.
Solar panels, structures, star trackers, reaction wheels, radios, flight software, avionics, launch dispenser — all built in-house.
Proliferated architectures demand production at scale. Rocket Lab is all in on SDA's mission, and the action on our floor proves it. We're proud to be delivering this.


🚀 Production line unlocked. Electron every 8 days. Rocket Lab hiring for a big 2027.
Let’s go! $RKLB!
Every 8 days an Electron rocket rolls off the production line thanks to our mission-obsessed team and advanced factories.
The Electron team is growing as we prepare to launch more rockets than ever before in 2027.
Role open across vehicle assembly, composites, GNC, propulsion, manufacturing engineering, software, and more. Those with automotive, aerospace, marine, aviation, and manufacturing experience are a great fit.
Come to New Zealand and Long Beach, CA to design, build, test, and launch rockets. Relocation support available.
Adventure awaits: rocketlabcorp.com/careers/
$ONDS Institutional Ownership Update
• 523 institutional holders
• 320.7 million shares held
Notable institutional holders include:
• BlackRock, Inc.
• Vanguard Capital Management LLC
• State Street Corp.
• VTSMX – Vanguard Total Stock Market Index Fund
• Geode Capital Management, LLC
• Vanguard Portfolio Management LLC
• Susquehanna International Group, LLP
• Hood River Capital Management LLC
• Citadel Advisors LLC
• Morgan Stanley
Data source: Source: Fintel
The long-term institutional accumulation trend speaks for itself.
THINKREAL 🎃
